From the brain’s movement and sensory areas to regions involved in higher-order association, white matter tracts do not all cross the same territory. Some remain within similar levels of the cortical hierarchy, while others stretch across it. That difference tracks with the range of cognitive functions associated with the tracts: the more of the hierarchy a tract spans, the more diverse its cognitive profile.
The finding emerged from an effort to describe white matter tracts not simply by familiar categories such as association or projection fibers, but by where their cortical endpoints sit within the brain’s broader organization.
The cortex can be arranged along a sensorimotor-to-association, or S–A, axis. At one end are regions involved in primary sensory and motor processing. At the other are higher-order association regions. The researchers asked whether major anatomical white matter tracts differ systematically in how far they extend along this hierarchy, and whether that positioning is related to the functions associated with them.
To make that comparison, the researchers used a population-level tract-to-region connectome built from diffusion MRI tractography in 1,065 young adults from the Human Connectome Project Young Adults dataset. The atlas contained 52 major white matter tracts, 26 in each hemisphere, and mapped each tract to 360 cortical regions from the HCP multimodal parcellation. A tract-to-region connection was counted when its connection probability reached at least 0.5 across the population.
This approach differs from a conventional structural connectome, which represents the brain mainly as pairs of connected regions. Here, the researchers retained the identity of the anatomical tract connecting multiple cortical regions. The tract definitions came from an atlas based on tractography with trajectory-based recognition and topology-informed pruning.
For each tract, the researchers calculated the average three-dimensional distance between its connected cortical regions. They also calculated its S–A range, defined as the difference between the highest and lowest S–A rankings among those regions. A larger range therefore meant that a tract reached across more of the cortical hierarchy.
The two measures were closely related. Tracts spanning greater physical distances also tended to span more of the cortical hierarchy, with a Spearman correlation of 0.688 and a permutation-test probability below 0.001 based on 10,000 iterations. The result indicated that shorter connections tended to join regions at similar hierarchical levels, whereas longer connections were more likely to bridge sensorimotor and association regions.
Each tract has its own cognitive profile
The researchers next asked what those anatomical differences might look like in terms of cognition.
They combined the tract-to-region maps with information from 125 cognitive terms drawn from the Cognitive Atlas and associated with meta-analytic functional MRI results in Neurosynth. For each cortical region, the analysis represented how strongly its activity was associated with each term. The researchers then linked those regional cognitive profiles to the white matter tracts reaching those regions.
A partial least-squares analysis identified a shared spatial pattern between cortical cognitive maps and tract connectivity. The significant latent variable explained 47.2% of the covariance between the two datasets. Its relationship also survived a spatially constrained cross-validation designed to account for spatial autocorrelation, with a median out-of-sample correlation of 0.65 that exceeded the corresponding spatially constrained null distribution.
The resulting pattern separated groups of tracts according to the cognitive functions associated with their cortical endpoints. The uncinate fasciculus, the paraolfactory segment of the cingulum and the anterior corticostriatal tract were associated particularly with affective functions such as mood, risk and emotion. The superior longitudinal fasciculus, middle longitudinal fasciculus and posterior corticothalamic tract were more strongly associated with goal-directed and action-related functions, including movement, imagery and action.
The researchers then calculated a more detailed cognitive profile for every tract by averaging its connected regions across all 125 terms.
The profiles were not interchangeable. The left arcuate fasciculus, for example, showed a strong association with language while also extending across other cognitive categories. The right arcuate fasciculus showed widespread involvement without the same language enrichment. The corticospinal tract had a strong motor and movement profile but was also associated with imagery and coordination. The uncinate fasciculus was dominated by emotion-related functions, while the vertical occipital fasciculus was associated particularly with attention and perception.
The widest-ranging tracts were also the most cognitively diverse
The researchers wanted to distinguish tracts that were associated mainly with a narrow group of functions from those with broader profiles.
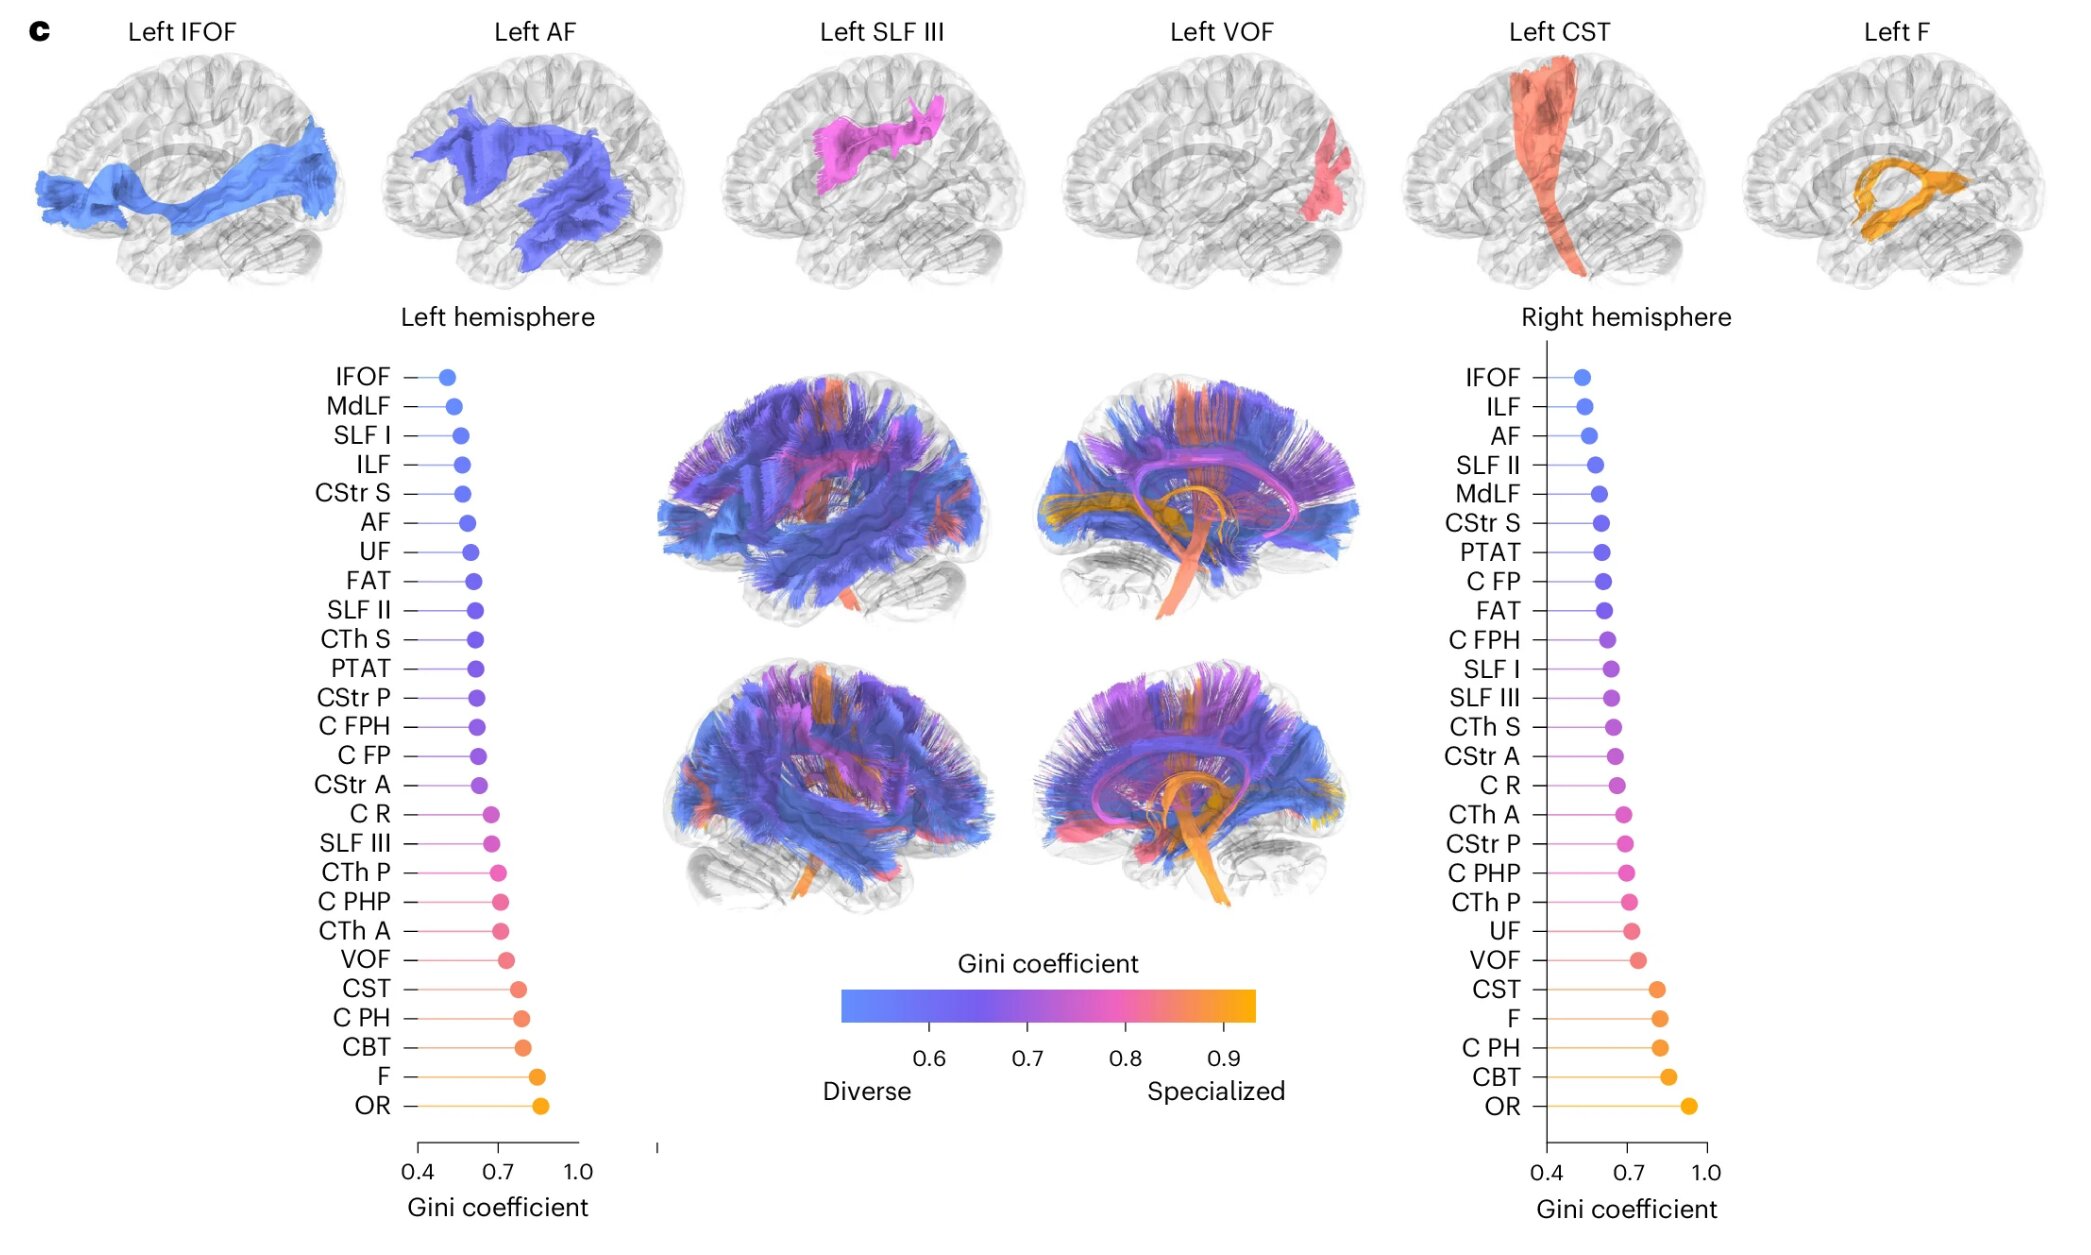
They used a Gini coefficient calculated across the 125 individual cognitive terms. A high Gini value indicated that a small number of terms dominated a tract’s profile, corresponding to greater specialization. A low value indicated a more even distribution across terms and therefore greater cognitive diversity.
The most specialized tracts included the optic radiation, fornix and corticobulbar tract. Among the most cognitively diverse were the inferior fronto-occipital fasciculus, middle longitudinal fasciculus and inferior longitudinal fasciculus.
The relationship between cognitive diversity and hierarchical position was strong. Across all 52 tracts, S–A range and the Gini coefficient were negatively correlated, with a Spearman correlation of −0.700 and a permutation-test probability below 0.001. In other words, tracts that reached across more of the sensorimotor-to-association hierarchy tended to have more evenly distributed and diverse cognitive profiles, whereas tracts connecting regions at similar hierarchical levels tended to be more specialized.
The relationship remained when the researchers analyzed projection and association tracts separately. For projection tracts, the correlation was −0.648, with a permutation-test probability of 0.002. For association tracts, it was −0.597, with a probability below 0.001. A separate tract-rewiring analysis, in which the researchers randomized tract connections while preserving the number of cortical regions connected by each tract and the hemisphere, also produced a correlation of −0.700, with a rewiring probability of 0.01 across 10,000 null networks.
The researchers also compared S–A range with the average S–A position of a tract. Across the analyses, S–A range was more consistently related to physical distance, cognitive diversity and cortical biological similarity. They therefore treated hierarchical span, rather than simply the average location of a tract, as the more informative description of its position in cortical organization.
Tracts also connect different biological environments
The cognitive pattern was accompanied by a difference in the biological properties of the cortical regions connected by each tract.
The researchers assembled 28 cortical feature maps covering properties including intracortical myelination, laminar characteristics, gene-expression patterns and neurotransmitter receptor distributions. They calculated the similarity of these biological profiles for pairs of cortical regions and then averaged the similarities for the regions connected by each white matter tract.
The differences were substantial. The vertical occipital fasciculus, for example, connected regions with relatively homogeneous biological profiles. The inferior fronto-occipital fasciculus connected regions with more heterogeneous profiles.
Across the tracts, greater S–A range was associated with lower mean cortical similarity. The Spearman correlation was −0.649, with a permutation-test probability below 0.001. The relationship was also present when projection and association tracts were examined separately, with correlations of −0.762 and −0.462, respectively. A tract-rewiring analysis produced a correlation of −0.649, again with a probability below 0.001.
Cognitive diversity showed a related pattern. Tracts with lower Gini coefficients, indicating more diverse cognitive profiles, tended to connect cortical regions with less similar biological properties. The correlation between Gini coefficient and mean cortical similarity was 0.599, with a permutation-test probability below 0.001. The authors therefore interpreted the results as evidence that some tracts connect relatively similar cortical environments, while others bridge regions that differ across multiple biological properties.
This pattern also provides a way to frame the relationship between anatomy and cognitive diversity. A tract that remains within a relatively narrow portion of the cortical hierarchy tends to connect regions with more similar biological characteristics and has a more specialized cognitive profile. Tracts extending across the hierarchy tend to encounter more heterogeneous cortical environments and have broader cognitive associations. The study demonstrates these relationships at the level of tract organization, but it does not establish that biological heterogeneity itself causes cognitive diversity.
The pattern appears during childhood and adolescence
The researchers then moved from population-level tract organization to individual differences in brain development.
They examined 1,145 participants in the Philadelphia Neurodevelopmental Cohort, ages 8 to 23. For 32 tracts available for this part of the analysis, they used diffusion MRI to measure fractional anisotropy, or FA, a measure of how strongly water diffusion is directionally constrained within white matter. Generalized additive models related tract FA to age while accounting for sex and head motion.
FA was significantly associated with age in 30 of the 32 tracts, or 93.8%, after false-discovery-rate correction. Effect sizes, expressed as partial R² values, ranged from −0.009 to 0.321 among significant tracts, and all but one tract showed a positive association between FA and age.
The size of those age-related effects was itself related to where the tracts sat in the cortical hierarchy. Tracts with greater S–A range had larger age-related FA effects, with a correlation of 0.708 and an FDR-corrected permutation probability below 0.001. Age effects were also larger in tracts with greater cognitive diversity, reflected by a negative correlation of −0.445 with the Gini coefficient.
The researchers tested the developmental pattern in an independent sample from the Healthy Brain Network, which included 638 participants ages 5 to 22. The relationship between age-related FA effects and S–A range was again positive, with a correlation of 0.666 and an FDR-corrected permutation probability below 0.001. The association with cognitive diversity was again negative, with a correlation of −0.375 and a probability of 0.03.
The HBN data allowed the researchers to examine additional measures of white matter microstructure. Mean diffusivity did not show the same consistent relationships with S–A range or cognitive diversity. Intracellular volume fraction, however, showed the same general pattern as FA, with a positive association with S–A range of 0.398 and a negative association with Gini coefficient of −0.640.
The researchers interpreted these findings as evidence that the tracts spanning the cortical hierarchy show stronger developmental variation during childhood and adolescence. They proposed that prolonged refinement of association cortex might contribute to changes in connected white matter, but explicitly described this as a speculation rather than a demonstrated mechanism.
Similar tract features are associated with individual differences in cognition
The final analysis examined whether the same anatomical organization was related to differences in cognitive performance.
In the Philadelphia Neurodevelopmental Cohort, the researchers focused on executive efficiency, a measure combining speed and accuracy across tasks involving executive functions such as attention and working memory. They again modeled tract FA while accounting for age, sex and motion.
FA was significantly associated with executive efficiency in 22 of the 32 tracts, or 68.8%, after FDR correction. All significant partial R² effects were positive, ranging from 0.004 to 0.023.
More importantly for the study’s central framework, the size of the cognition-related FA effects was positively associated with S–A range. The correlation was 0.495, with an FDR-corrected permutation probability of 0.006. The association with Gini coefficient was negative, at −0.377 with a probability of 0.037. Thus, tracts spanning more of the cortical hierarchy and having more diverse cognitive profiles showed stronger relationships between individual differences in FA and executive efficiency.
The researchers replicated the analysis in 1,097 adults from the Human Connectome Project Young Adults, ages 22 to 37. In that dataset, cognition was measured using the NIH Toolbox fluid cognition composite.
The same pattern appeared. The association between tract FA and cognitive performance was positively related to S–A range, with a correlation of 0.587 and an FDR-corrected permutation probability of 0.001. It was negatively related to Gini coefficient, with a correlation of −0.601 and a probability of 0.001.
The researchers also tested mean diffusivity in these cognition analyses. Unlike FA, MD did not show consistent relationships with either S–A range or cognitive diversity. In the PNC, the correlations between MD-related cognition effects and S–A range and Gini coefficient were −0.08 and 0.02, respectively. In HCP-YA, they were −0.329 and 0.435, with neither set meeting the study’s FDR-corrected significance criteria.
The findings come with important limits
The relationships described in the study are based largely on population-level tract-to-cortex maps rather than individualized maps of every person’s tract endpoints. The authors note that although most tract-to-region connection probabilities were close to either zero or one, there is still interindividual variation in those connections.
The developmental and cognition analyses were also restricted to 32 of the 52 tracts because of changes in the white matter atlas used for those measurements. The overall tract-to-region analysis included 52 major tracts, but the individual-difference analyses therefore covered a smaller subset.
Tractography itself is an approximation. The authors note that diffusion MRI tractography has limitations in representing the complex fiber dispersion and branching observed in anatomical tracing studies. The study also excluded certain tract types, including commissural, brainstem and connections between subcortical structures, because of methodological limitations.
The interpretation of FA requires particular caution. FA reflects the degree to which water diffusion is directionally constrained, but it can be influenced by crossing fibers, fiber diameter and density, and myelination. The authors therefore do not treat age-related or cognition-related FA differences as a direct measure of a single biological process.
The developmental datasets were cross-sectional rather than longitudinal, so the analyses cannot establish how individual white matter tracts change within the same person over time. The authors identify longitudinal studies as an important next step, along with analyses that determine whether tract-to-region connections themselves change across the lifespan.
The cognitive annotations also describe associations between tracts and functions rather than demonstrating that an individual tract causes a particular cognitive ability. The researchers’ framework links anatomical tracts to the functions associated with their cortical endpoints, but it does not by itself establish a causal pathway from tract anatomy to behavior.
The resulting picture is therefore not that every long-range white matter tract has the same role. Instead, the 52 tracts occupy different positions relative to the sensorimotor-to-association organization of the cortex. Some connect regions close to one another in that hierarchy and have relatively specialized cognitive profiles. Others span a much broader portion of the hierarchy, connect cortical regions with more heterogeneous biological properties, and show broader cognitive associations. Those same hierarchy-spanning tracts also showed stronger relationships with developmental variation in white matter microstructure and with individual differences in cognition across the datasets examined.
The authors propose extending this framework to additional tract classes, including commissural and subcortical pathways, as well as short U-fibers. They also call for longitudinal developmental studies, age-specific tract-to-region maps and investigations of individual variation in tract endpoints.
The study was published in Nature Human Behaviour.